Nitrogen-Fixing Bacteria
Historical document, translated for reference. It reflects medical knowledge of the 1920s–30s and is not medical advice.
Summary
An overview of nitrogen-fixing bacteria from the 1928-1936 Great Medical Encyclopedia, detailing root nodule bacteria in symbiosis with legumes as well as free-living aerobic and anaerobic soil species.
Encyclopedia article (1928–1936)
NITROGEN-FIXING BACTERIA, bacteria capable of feeding on free atmospheric nitrogen, which is entirely unsuitable for the nutrition of most microbes. Two groups of nitrogen-fixing bacteria are known: some of them, the so-called "nodule bacteria," fix nitrogen in symbiosis with leguminous plants, forming special swellings or nodules on their roots; the other group of nitrogen-fixing bacteria vegetates freely in the soil and is not directly dependent on the life of higher plants. Among the representatives of the second group of nitrogen-fixing bacteria, there are aerobic and anaerobic species, which are very widespread in nature. Nodule bacteria were discovered and studied earlier. The discovery of
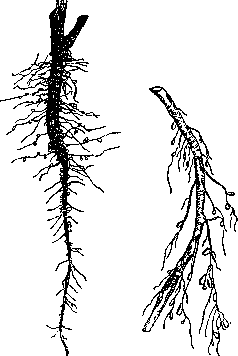
Figure 1. Root of Vicia faba with young nodules.
Figure 2. Root of Trifolium pratense with nodules. This group of nitrogen-fixing bacteria was preceded by ancient and very interesting observations from agricultural practice. It was noted that in relation to nitrogen nutrition, all cultivated plants can be divided into two groups, unequal in the number of representatives. While the vast majority of plants, including all cereals, require combined nitrogen for their nutrition and, absorbing nitric acid salts through their roots, deplete the nitrogen reserve in the soil, other plants belonging to the legumes grow exceptionally well on nitrogen-poor soils, not only without exhausting them, but, on the contrary, improving their quality and enriching them with nitrogen. The discovery of the two groups of plants—those that exhaust and those that enrich the soil with nitrogen—served as the basis upon which the modern doctrine of crop rotation grew. Research by Hellriegel and Wilfarth established that there is a mutual relationship between the presence of special wart-like growths on the roots of legumes, the so-called "root nodules" (see figures 1 and 2), and the fixation of free nitrogen by these plants. When a sterilized bean is sown in sterilized soil, nodules do not appear at all. In this case, in the absence of combined nitrogen in the soil, legumes develop just as poorly as cereals. If, however, in a parallel experiment, the same but unsterilized
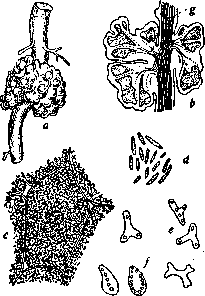
Figure 3. Root nodules of legumes: a—lupine nodules in natural size; b—longitudinal section of a lupine root with a nodule; v—vascular bundle of the root; s—cell of the lupine nodule packed with bacteria; d—nodule bacteria in unchanged form; e, f—bacteroids (magnification: s—600; d, e, f—approx. 1,500).
soil is taken, the legume will develop quite normally with abundant nodule formation. The latter develop especially profusely in soils poor in combined nitrogen, giving the roots of the legume their characteristic appearance. If, however, the legume is provided with nitrogenous nutrition, the nodules either do not appear at all or develop poorly. They should therefore be regarded merely as a temporary adaptation used by the legume to fix atmospheric nitrogen, which is not part of the normal development cycle of this plant when there is a sufficient content of nitrates in the soil. As the legume grows, the nodules become drier, wrinkle, and gradually disintegrate, giving their accumulated reserve of nitrogen to the plant, with whose vascular bundles they are in direct connection (see figure 3). In some legumes (peas, clover, vetch), nodules form as small swellings on the fine branches of the roots and on rootlets (see figure 1); in others, conversely, e.g., in lupine, they cover the main root of the plant with large wart-like growths, sometimes reaching the size of a hazelnut (see figure 3). In young nodules, the bacteria appear as unusually small, non-spore-forming, highly motile rods. As the nodule develops, the bacteria increase in size, and "bacteroids" appear among them (see figure 3, e and f). The appearance of bacteroids is a sign of incipient degeneration under the influence of the processing of bacteria by the acidic juices of the host plant, which is in the period of full development. The remains of disintegrated nodules infect the soil with surviving bacteria, and therefore soils from under legume cultivation are usually rich in nodule bacteria. Bacteria isolated from the nodules of various legumes are almost identical in their morphological and cultural characteristics, and therefore they are all united into a common species—Bac. radicicola, distinguishing only individual races. However, physiologically these varieties differ quite substantially in that each of them causes abundant nodule formation only on the roots of its own host plant. Only through systematic experiments is it possible to acclimate nodule bacteria to other legumes and thus obtain "crossing microbes," but this mutual exchange of host plants succeeds only between closely related species, e.g., between clover and alfalfa, between beans and vetch, etc. The symbiosis of the legume with nodule bacteria bears the features of a kind of mutual parasitism: at first the bacteria parasitize the plant, utilizing nutrients, and then the plant returns its losses with interest, taking from the bacteria a mucous nitrogenous substance that serves for nutrition. Direct observation convinces us that the soil itself possesses nitrogen-fixing powers, and that along with nodule bacteria, other groups of microbes also exist in the soil layer that perform the same process of nitrogen fixation independently of the cultivation of leguminous plants. They were discovered in 1893 by Winogradsky, who used a nitrogen-free medium for their isolation, containing, along with necessary mineral nutrients, a large amount of sugar, the decomposition of which serves as a energy source for the microbes. Winogradsky Figure 4. Development scheme of Clostridium Pasteurianum: 1—rods; 2—spindle-shaped form; 3—spore formation; 7—mature spore with a characteristic triangular sheath (cell remnant); 8—spore germination. managed thus to obtain in anaerobic conditions a pure culture of the nitrogen-fixing rod, which he named Clostridium Pasteurianum (see figure 4). This is a fairly large anaerobic species that takes on the form of a short spindle during the spore-formation period and stains blue with iodine at this stage. In the mature state, the elongated spore is surrounded by the remnant of the body of the bacillus in the form of a gelatinous triangular sheath. The spore germinates polarly and always from the open side of the sheath. The distribution of Clostridium Pasteurianum in nature is very wide. It was isolated from Figure 5. 1—Azotobacter chroococcum; 2—Azotobacter agile (magnification 1,000). a wide variety of soils of the Old and New Worlds. Clostridium Pasteurianum causes typical butyric acid fermentation in sugary liquids with the formation of butyric and acetic acids, butyl alcohol, hydrogen, and carbon dioxide; its nitrogen fixation, according to Winogradsky, occurs through the formation of ammonia from atmospheric nitrogen and nascent hydrogen. The reduced ability to fix nitrogen can be restored to its previous size if the microbe is "passed through the soil" by sowing a weakened culture into sterilized soil, much like the virulence of pathogenic microbes is restored by passing them through the organism of a susceptible animal. In 1901, Beijerinck isolated from garden soil an aerobic species—Azotobacter chroococcum—in the form of large, slightly elongated cells with a sharply expressed property of fixing atmospheric nitrogen (see figure 5, 1). Simultaneously, a variety Azotobacter agile, of somewhat larger size, was isolated by him from sewage water (see figure 5, 2). Azotobacter cells are usually provided with a mucous capsule, sometimes exceeding the size of the bacterial body itself. In the division stage, the cells appear as large diplococci. Their protoplasm possesses a clearly expressed granularity. Like Clostridium Pasteurianum, Azotobacter fixes nitrogen only in the presence of nitrogen-free organic substances, which it burns to the end. The mechanism of fixation is, in all probability, the same as that of Clostridium Pasteurianum. The nitrogen assimilated by Azotobacter is deposited in its body in the form of protein compounds. Upon entering the soil, Azotobacter cells undergo successive processes of putrefaction and nitrification, and their nitrogen thus becomes available for the nutrition of higher plants. Azotobacter is extraordinarily widespread in various soils. Intensive plowing of the land, which facilitates the access of air to it, as well as the addition of lime salts, favors the development and activity of Azotobacter. A weakly expressed property of binding atmospheric nitrogen is also possessed by some other species of microorganisms (bacteria, algae, fungi) that are very widespread in nature.
Related articles
Mentioned in
Cite this page
“Nitrogen-Fixing Bacteria.” Soviet Medical Encyclopedia. English translation of Bolshaya Meditsinskaya Entsiklopediya, 1st ed. (Moscow, 1928–1936), ed. N. A. Semashko. https://sovietmedicalencyclopedia.com/article/nitrogen-fixing-bacteria/