Agglutination
Historical document, translated for reference. It reflects medical knowledge of the 1920s–30s and is not medical advice.
Summary
This article provides a detailed overview of the phenomenon of agglutination, covering its immunological definition, the role of agglutinins and agglutinogens, and various physicochemical theories explaining the mechanism of bacterial clumping. It discusses historical perspectives from the early 20th century, including the work of Ehrlich, Gruber, Durham, and others.
Encyclopedia article (1928–1936)
AGGLUTINATION, the precipitation of bacteria or other cellular elements upon exposure to the serum of an animal that is insusceptible (immune) to them. The property of serum to cause agglutination is explained by Ehrlich's theory (see Immunity) as the accumulation within it, during the course of immunization, of special substances that have received the name "agglutinins." The agglutination reaction was first studied by Gruber and Durham (1896). In the blood serum of a healthy person, normal agglutinins are also sometimes found in relation to individual species of bacteria, for example, typhoid, dysentery, etc. In early childhood (Landsteiner), there are no normal agglutinins. Apparently, they are formed at a more mature age as a result of imperceptible immunization of the organism by the corresponding bacteria through the intestinal wall or by another route. The impetus for the accumulation of agglutinins is either the infection of the animal, or the artificial introduction into it of live and killed cultures of microbes (resp. foreign cells), or, finally, the same introduction of microbial proteins. Substances capable, upon parenteral administration, of causing the formation and accumulation of agglutinins in the organism are called agglutinogens (see Antigens). The protein molecule of an agglutinogen has an insignificant size and is capable of passing through a colloidal filter. Agglutinogen is contained in bacterial cultures in a dissolved state, and there is more of it in old cultures than in young ones. Agglutinogen is not destroyed by treatment with formalin or by boiling. Bacteria are killed in this process, but they retain the ability to be agglutinated and to cause the formation of agglutinins in the organism of animals. Sera have a larger particle than agglutinogen and do not pass through a colloidal filter. Agglutinins are bound predominantly to the euglobulin fraction of blood serum, and to a lesser extent to the pseudoglobulin fraction. They are destroyed by heating to 60–65°; alkalis destroy them easily; acids are harmful to a lesser degree. Alexin or complement (see Alexin) does not play a significant role in the agglutination reaction. The bacterial cell represents a complex conglomerate of proteins. Some of these proteins may be common to bacteria belonging to one and the same phylogenetic group. Hence it is understandable that an agglutinating serum, specific for one species of bacteria, will agglutinate, although more weakly, other species of bacteria that are related and belong to the same group as the first. Such related agglutination is called group agglutination. Finally, some cultures of bacteria possess the ability for spontaneous agglutination in physiological saline (autoagglutination) without any immune or normal serum. According to Ehrlich's terminology, agglutinins have a haptophore group, which fixes them to bacteria, and a toxophore or ergophore group, which causes the phenomenon of clumping-agglomeration and precipitation-agglutination. Degeneration of the toxophore group of the agglutinin leads to the formation of agglutinoids. The inactivation of agglutinins and their conversion into agglutinoids occurs upon heating to 58–70°. Various chemical substances, such as salts, alkalis, acids, formalin, and uric acid, also destroy the ergophore group of agglutinins. Bacteria saturated with the corresponding agglutinoid lose the ability for agglutination. The essence of agglutination, from the point of view of physical chemistry, consists of the following. Bacteria are uniformly distributed in a liquid during active, or Brownian, molecular motion due to the fact that their bodies carry a uniform electrical charge. In an electric current, bacteria move toward the anode; consequently, they are negatively charged. At the same time, bacteria possess a force of mutual attraction, which depends on surface tension. It is obvious that with uniform distribution in a liquid, the repulsive force is greater than the force of attraction. Agglutination occurs at the moment when the uniform electrical charge is weakened to such a degree that the force of attraction gains the upper hand. An increase in the force of attraction can also be accompanied by agglutination. Bacteria are agglutinated at the moment when the potential difference drops below 15 millivolts (Northrop and De Kruif), provided the force of attraction of the bacteria remains constant. In the event that the force of attraction decreases or becomes very small, agglutination does not occur even when the potential is reduced to zero. The origin of the potential can be explained on the basis of Donnan's theory, according to which in protein liquids separated by a colloidal membrane, permeable to all ions of one liquid and part of the ions of the other, a potential difference arises, the magnitude of which depends on the concentration and charge of the components of the liquid. Bordet (1899) classifies agglutination among the phenomena of the precipitation of colloidal particles from a suspension (dispersion) in a liquid under the influence of electrolytes. Bacteria and agglutinating serum, freed from salts by dialysis, do not exhibit the phenomenon of agglutination even upon prolonged standing. The addition of traces of an electrolyte—NaCl—to such a mixture immediately causes the agglutination of bacteria. The binding of agglutinin by bacteria also occurs in the absence of salt: bacteria loaded with agglutinins can be centrifuged, washed of serum, and suspended in distilled water. The addition of traces of salt to such a suspension of bacteria immediately causes the agglutination of the bacteria. Agglutination occurs not only in the presence of NaCl, but also of many other salts, as well as crystalloids of an organic nature (Friedberger). The agglutination reaction, upon the subsequent addition of an electrolyte, proceeds in the same way as in a mixture of two colloids carrying electrical charges of opposite character, where one of the colloids is present in a smaller quantity and is not in a condition to completely neutralize the charge of the other. In such a case, the addition of an electrolyte, which splits in solution into salt ions, contributes to the complete neutralization of the electrical charge of the predominant colloid. Neutral particles of colloids, by virtue of surface tension and mutual attraction, precipitate in the form of flakes. Agglomeration of suspensions, which bacteria are, is also possible with the help of the combined action of a colloid and an electrolyte. A suspension of mastic, in the presence of a small amount of gelatin or protein-containing liquids, is precipitated by the addition of traces of salt (Neisser and Friedemann). Experiments of this kind prove with certainty the physicochemical (colloidal) nature of the agglutination reaction. To neutralize one colloid with another, a specific quantitative ratio of their electrical charges is necessary. With an excess of one of them, a predominance of a charge of the opposite character arises, consequently, a recharging of the colloid and, in connection with this, a stabilization of its dispersed state. In this way, "zones of inhibition" of the reaction arise. They often take place during the agglutination of bacteria with fresh sera that do not contain agglutinoids. In such a case, the agglutinating serum in concentrated dilutions sometimes does not agglutinate or gives a weak reaction, while at higher dilutions the reaction is clearly expressed. The explanation of the essence of the agglutination reaction by the neutralization of the electrical charges of colloids met with objections from Michaelis and Davidson, who found that the agglutination reaction can occur with large fluctuations in the concentration of H-ions. The optimum of the reaction does not coincide with the isoelectric point of the antigen and agglutinin. Therefore, Dean proposed another theory, according to which, during the process of agglutination, bacteria adsorb particles of the agglutinin colloid, which are deposited on their surface. Antigen proteins that have emerged into the surrounding liquid and bind the globulins of the immune serum also participate in this process. By virtue of a change in surface tension, agglutination of the bacteria occurs; they become visible to the eye in clumps and then, by virtue of gravity, settle to the bottom. The enzymatic theory of agglutination was first proposed by Mansfield (1918), who interpreted the reaction in the following way: bacteria are held in suspension thanks to protective colloids (agglutinin contains an enzyme that destroys this membrane and the antigen itself). As a consequence of this, bacteria, not protected by a membrane, positively or negatively charge the salt ions of the solution, lose their uniform electrical charge, and, mutually attracting one another, gather into clumps and precipitate. Zdravomyslov (1924) presents the participation of the enzyme in the process of agglutinin formation differently: under experimental conditions, agglutinins are obtained by mixing antigen with trypsin. As a result of the digestion of bacterial proteins, a trypsinate is obtained, in which agglutinins are contained, which should be considered as an enzyme bound by the products of the breakdown of bacterial proteins. Physicochemical theories have not yet provided an explanation for the specificity of immunity reactions. An analogy to the specificity of serum agglutination is presented by the acid agglutination of bacteria (Michaelis), based on the fact that the concentration of H-ions at which a protein precipitates is specific for each of them. Therefore, the agglutination of bacteria by acids occurs at a specific concentration of H-ions for each species of microorganism. This reaction is, however, not to the same degree specific as the reactions of immunity (Gouwens, 1923). The role of agglutinins in immunity is unclear.
Agglutinated bacteria do not lose their viability and continue to multiply at the bottom of a vessel with a nutrient medium. Typhoid bacteria in agglutinating serum grow in the form of flakes consisting of filaments (Mandelbaum). The laboratory use of agglutinins is possible in two directions: 1) to establish a diagnosis of a disease, the patient's blood serum is used, which is mixed in certain dilutions with a culture of known bacteria—the diagnosis of the disease is made on the basis of the presence of corresponding agglutinins in the blood (see Widal reaction); 2) a specific agglutinating serum is mixed with a culture of an unknown microorganism—on the basis of the presence of agglutination, the identification of the species of the microorganism is made. The agglutination reaction has practical application in the recognition of typhoid fever, paratyphoid infections, bacillary dysentery, Malta fever, meningitis, and some other infections. In such cases, the agglutination reaction is conclusive if the specific immune serum agglutinates the given culture in dilutions close to its titer. The titer of the serum is called that smallest amount of it which still possesses agglutinating action. The result of the agglutination reaction can be determined in a sharply pronounced reaction with the naked eye or, better, with a magnifying glass, and most clearly with an agglutinoscope (Kuhn and Woithe), which allows for determining the size of the flakes. Group agglutinins can be distinguished from the main ones with the help of the Castellani experiment, based on the fact that bacteria bind all agglutinins of the immune serum for a given species. Group agglutinins are also bound in this process. If the serum is brought into contact with a species of bacteria other than the one with the help of which it was produced in the animal's organism, then the main agglutinins remain free. NaCl solutions of increased concentration (2.9–5.8%) in the Widal reaction suppress group agglutination.
M. Shtutser. Agglutinoscope, an apparatus for observing the phenomenon of agglutination. The most convenient is the Kuhn-Woithe model. As can be seen from the figure, the test tube with the liquid is inserted into a metal tube having an opening
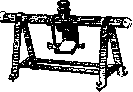
opposite the magnifying glass. Light rays reflected from a mirror, passing through the test tube, are deflected by the formed clusters and allow one to see the smallest flakes, inaccessible to the naked eye. At the present time, the agglutinoscope is also partly used for reading flocculation reactions (Meinicke, Sachs-Georgi, etc.).
Related articles
Mentioned in
- Active Immunization
- Agglutinating Sera
- Aggravation
- Antibodies
- Antigens
- Belonovsky, Georgy Dmitrievich
- Bizzozero's Plaques
- Coagglutination
- Cross-Immunization
- Erythrocyte Sedimentation
- False Agglutination
- Gruber
- Hanging Drop
- Hemagglutination
- Hyponoic Mechanisms
- Immunobiological Reactions
- Isoreactions
- Jules Bordet
- Maltese Fever
- Paraagglutination
Cite this page
“Agglutination.” Soviet Medical Encyclopedia. English translation of Bolshaya Meditsinskaya Entsiklopediya, 1st ed. (Moscow, 1928–1936), ed. N. A. Semashko. https://sovietmedicalencyclopedia.com/article/agglutination/